Anti-Cdk1 (Tyr-15) [conserved site], Phosphospecific Antibody (M231)
Our Cdk1 (Tyr-15)[conserved site] phosphospecific primary antibody from PhosphoSolutions is mouse monoclonal. It detects human, mouse, and rat Cdk1 (Tyr-15)[conserved site] and is Protein A purified. It is great for use in WB.
SKU: CM2311
Ships: 1-2 business days
Product Details
Cdk1 (Tyr-15)[conserved site]
Cyclin-dependent kinases (Cdks) are a family of serine/threonine kinases that require association with regulatory subunits known as cyclins for activation. In addition, post-translational phosphorylation and dephosphorylation events regulate Cdk activity. Phosphorylation of Thr-160 in the T loop by Cdk-activating kinase (CAK) is an obligatory step in kinase activation. By contrast, phosphorylation of the Thr-14 and Tyr-15 residues by the Wee1 family of dual specificity kinases is inhibitory for the Cdks, and dephosphorylation of these residues by the Cdc25 family of phosphatases coincides with Cdk activation. Alternatively, Cdk5 appears to require different mechanisms for activation. This Cdk is activated through association with specific activators, including p35, p39, and p67. Cdk5 is primarily activated in neuronal cells, and only c-Abl kinase, rather than Wee family members, have been shown to phosphorylate Tyr-15 to regulate its activity.
Protein A Purified
Monoclonal
M231
IgG1
ELISA, WB
Mouse
CDK1
34
Clone M231 was generated from a phospho-Cdk1 (Tyr-15) synthetic peptide (coupled to carrier protein) corresponding to amino acids surrounding Tyr-15 in human Cdk1. This sequence is conserved in rat and mouse Cdk1, and is highly conserved in other Cdks, including Cdk2, Cdk3, Cdk5, and Cdk6.
Human
Human, Mouse, Rat
Storage at -20°C is recommended, as aliquots may be taken without freeze/thawing due to presence of 50% glycerol. Stable for at least 1 year at -20°C.
Liquid
PBS + 1 mg/ml BSA, 0.05% NaN3 and 50% glycerol
WB: 1:250
Unconjugated
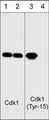
The antibody detects a 34 kDa* band corresponding to Cdk1 on SDS-PAGE immunoblots of human SYF and HeLa cells, and this band is removed after alkaline phosphatase treatment. The antibody may also detect Tyr-15 phosphorylation in Cdk2, Cdk3, Cdk5, and Cdk6.
Phosphorylated
Western blots performed on each lot.
For research use only. Not intended for therapeutic or diagnostic use. Use of all products is subject to our terms and conditions, which can be viewed on our website.
United States
After date of receipt, stable for at least 1 year at -20°C.
Cdc 2; Cdc2; Cdc2; CDC28A; CDK-1; CDK 1; CDK1; CDK1_HUMAN; CDKN1; CELL CYCLE CONTROLLER CDC2; Cell division control protein 2; Cell division control protein 2 homolog; Cell division cycle 2 G1 to S and G2 to M; Cell division protein kinase 1; Cell Divsion Cycle 2 Protein; Cyclin Dependent Kinase 1; Cyclin-dependent kinase 1; DKFZp686L20222; MGC111195; p34 Cdk1; p34 protein kinase; P34CDC2
P06493
UniProt Summary: Plays a key role in the control of the eukaryotic cell cycle by modulating the centrosome cycle as well as mitotic onset; promotes G2-M transition via association with multiple interphase cyclins. Phosphorylates PARVA/actopaxin, APC, AMPH, APC, ASB7, BARD1, Bcl-xL/BCL2L1, BRCA2, CALD1, CASP8, CDC7, CDC20, CDC25A, CDC25C, CC2D1A, CENPA, CSNK2 proteins/CKII, FZR1/CDH1, CDK7, CEBPB, CHAMP1, DMD/dystrophin, EEF1 proteins/EF-1, EZH2, KIF11/EG5, EGFR, FANCG, FOS, GFAP, GOLGA2/GM130, GRASP1, UBE2A/hHR6A, HIST1H1 proteins/histone H1, HMGA1, HIVEP3/KRC, UHRF1, KAT5, LMNA, LMNB, LBR, MKI67, LATS1, MAP1B, MAP4, MARCKS, MCM2, MCM4, MKLP1, MLST8, MYB, NEFH, NFIC, NPC/nuclear pore complex, PITPNM1/NIR2, NPM1, NCL, NUCKS1, NPM1/numatrin, ORC1, PRKAR2A, EEF1E1/p18, EIF3F/p47, p53/TP53, NONO/p54NRB, PAPOLA, PLEC/plectin, RB1, TPPP, UL40/R2, RAB4A, RAP1GAP, RBBP8/CtIP, RCC1, RPS6KB1/S6K1, KHDRBS1/SAM68, ESPL1, SKI, BIRC5/survivin, STIP1, TEX14, beta-tubulins, MAPT/TAU, NEDD1, VIM/vimentin, TK1, FOXO1, RUNX1/AML1, SAMHD1, SIRT2, CGAS and RUNX2. CDK1/CDC2-cyclin-B controls pronuclear union in interphase fertilized eggs. Essential for early stages of embryonic development. During G2 and early mitosis, CDC25A/B/C-mediated dephosphorylation activates CDK1/cyclin complexes which phosphorylate several substrates that trigger at least centrosome separation, Golgi dynamics, nuclear envelope breakdown and chromosome condensation. Once chromosomes are condensed and aligned at the metaphase plate, CDK1 activity is switched off by WEE1- and PKMYT1-mediated phosphorylation to allow sister chromatid separation, chromosome decondensation, reformation of the nuclear envelope and cytokinesis. Phosphorylates KRT5 during prometaphase and metaphase. Inactivated by PKR/EIF2AK2- and WEE1-mediated phosphorylation upon DNA damage to stop cell cycle and genome replication at the G2 checkpoint thus facilitating DNA repair. Reactivated after successful DNA repair through WIP1-dependent signaling leading to CDC25A/B/C-mediated dephosphorylation and restoring cell cycle progression. Catalyzes lamin (LMNA, LMNB1 and LMNB2) phosphorylation at the onset of mitosis, promoting nuclear envelope breakdown. In proliferating cells, CDK1-mediated FOXO1 phosphorylation at the G2-M phase represses FOXO1 interaction with 14-3-3 proteins and thereby promotes FOXO1 nuclear accumulation and transcription factor activity, leading to cell death of postmitotic neurons. The phosphorylation of beta-tubulins regulates microtubule dynamics during mitosis. NEDD1 phosphorylation promotes PLK1-mediated NEDD1 phosphorylation and subsequent targeting of the gamma-tubulin ring complex (gTuRC) to the centrosome, an important step for spindle formation. In addition, CC2D1A phosphorylation regulates CC2D1A spindle pole localization and association with SCC1/RAD21 and centriole cohesion during mitosis. The phosphorylation of Bcl-xL/BCL2L1 after prolongated G2 arrest upon DNA damage triggers apoptosis. In contrast, CASP8 phosphorylation during mitosis prevents its activation by proteolysis and subsequent apoptosis. This phosphorylation occurs in cancer cell lines, as well as in primary breast tissues and lymphocytes. EZH2 phosphorylation promotes H3K27me3 maintenance and epigenetic gene silencing. CALD1 phosphorylation promotes Schwann cell migration during peripheral nerve regeneration. CDK1-cyclin-B complex phosphorylates NCKAP5L and mediates its dissociation from centrosomes during mitosis. Regulates the amplitude of the cyclic expression of the core clock gene BMAL1 by phosphorylating its transcriptional repressor NR1D1, and this phosphorylation is necessary for SCF(FBXW7)-mediated ubiquitination and proteasomal degradation of NR1D1. Phosphorylates EML3 at 'Thr-881' which is essential for its interaction with HAUS augmin-like complex and TUBG1. Phosphorylates CGAS during mitosis, leading to its inhibition, thereby preventing CGAS activation by self DNA during mitosis. Phosphorylates SKA3 on multiple sites during mitosis which promotes SKA3 binding to the NDC80 complex and anchoring of the SKA complex to kinetochores, to enable stable attachment of mitotic spindle microtubules to kinetochores.
983
Blue Ice